Research Article
Outdoor Nursery Propagation of Kava (Piper methysticum) by Air Layering
A three-season trial of two American kava varieties under ambient subtropical nursery conditions in South Florida, with layer-level rooting outcomes, seasonal replication and a labor and materials accounting
- 1 American Kava Association; Root of Happiness, Las Vegas, Nevada, USA
- 2 American Kava Association; Nakamal at Home, Boca Raton, Florida, USA
Correspondence: Tyler Blythe, admin@americankavaassociation.org · ORCID: Tyler Blythe 0009-0006-7884-0650; Jeffrey Bowman 0009-0004-1269-6559
- DOI
- Pending Crossref registration
- Preprint
- 10.5281/zenodo.22838843 · AKA Technical White Paper No. 4
- Received
- 19 September 2026
- Accepted
- 28 October 2026
- Published
- 28 October 2026
- Volume
- Volume 1 (2026)
- Article
- 004
- Article type
- Research Article
- Review
- Computational Manuscript Review (CMR) · Editorially accepted
- Handling editor
- Tyler Blythe, Editor-in-Chief (also an author)
- License
- CC BY 4.0 · © 2026 The Author(s)
Abstract
This study evaluated air layering as a vegetative propagation method for Piper methysticum (kava) under ambient outdoor nursery conditions in South Florida across three seasonal replicates: June 2025 (summer wet season), October 2025 (fall transitional season), and February 2026 (winter dry season). In each replicate, forty air layers were established on two American kava varieties, Kali-ISA and Kali-Hiwa (n = 20 per variety per replicate), using auxin-treated, microbially inoculated sphagnum moss enclosed in opaque two-piece polypropylene pods. Layers were scored at 21 days on a standardized four-category rooting scale (rotted; alive, no roots; poorly rooted; well rooted). Pooled across replicates (n = 60 per variety; n = 120 total), rooting success was 81.7% (49/60; 95% CI 70.1–89.4) for Kali-ISA and 70.0% (42/60; 95% CI 57.5–80.1) for Kali-Hiwa, for an aggregate rate of 75.8% (91/120; 95% CI 67.4–82.6). The 11.7 percentage-point difference between varieties was not statistically significant (Yates-corrected χ² = 1.64, df = 1, p = 0.20; Mantel–Haenszel common odds ratio 1.92, 95% CI 0.81–4.52, p = 0.14), and no within-replicate comparison approached significance. Rooting also did not differ significantly across the three seasonal windows (χ² = 0.64, df = 2, p = 0.73), indicating that the method performed consistently under summer, transitional, and winter conditions rather than that any season was demonstrably superior. Aggregate rooting exceeded published outcomes for nodal stem cuttings in the South Pacific (20–60% plant establishment depending on node position and planting month [1]) and the authors' previously reported soft-stem propagation in peat cubes (47%) and aeroponics (51%) [2]; these are historical rather than concurrent controls and the endpoints are not strictly equivalent. All successfully rooted layers survived to the 30-day post-transplant assessment. Air layering appears to be a reproducible, low-infrastructure propagation option for American kava varieties under ambient subtropical nursery conditions. The design carries material limitations: a single site, no concurrent control or comparator arm, multiple layers per stock plant with within-plant clustering unmodeled, and no blinding of assessors. The results should be read as a proof of concept that warrants a controlled, adequately powered trial rather than as a demonstration of superiority over existing methods.
Keywords: Piper methysticum; kava; air layering; marcotting; vegetative propagation; adventitious rooting; sphagnum moss; microbial inoculant; South Florida; seasonal replication
1. Introduction
Vegetative propagation of Piper methysticum has historically relied on nodal stem cuttings taken from mature plants, a practice that constrains the availability of planting material and ties propagation cycles to harvest timing. Alternatives have been explored, including soft-stem propagation in peat cubes and aeroponic systems and tissue-culture micropropagation [2,3,4]. These methods generally require controlled environments, specialized infrastructure, or technical inputs that limit their use in low-infrastructure nursery and smallholder settings.
Air layering (marcotting) is widely used in other woody and tropical crops, including the economically important Piper species P. nigrum, P. betle, and P. longum. Its application to kava is described qualitatively in the monograph literature — Lebot and Cabalion [5] note that marcotting is straightforward in kava and that runner nodes contacting the ground root spontaneously — but we could locate no peer-reviewed study that quantifies air-layering outcomes in P. methysticum using standardized rooting criteria, or that benchmarks them against other kava propagation systems.
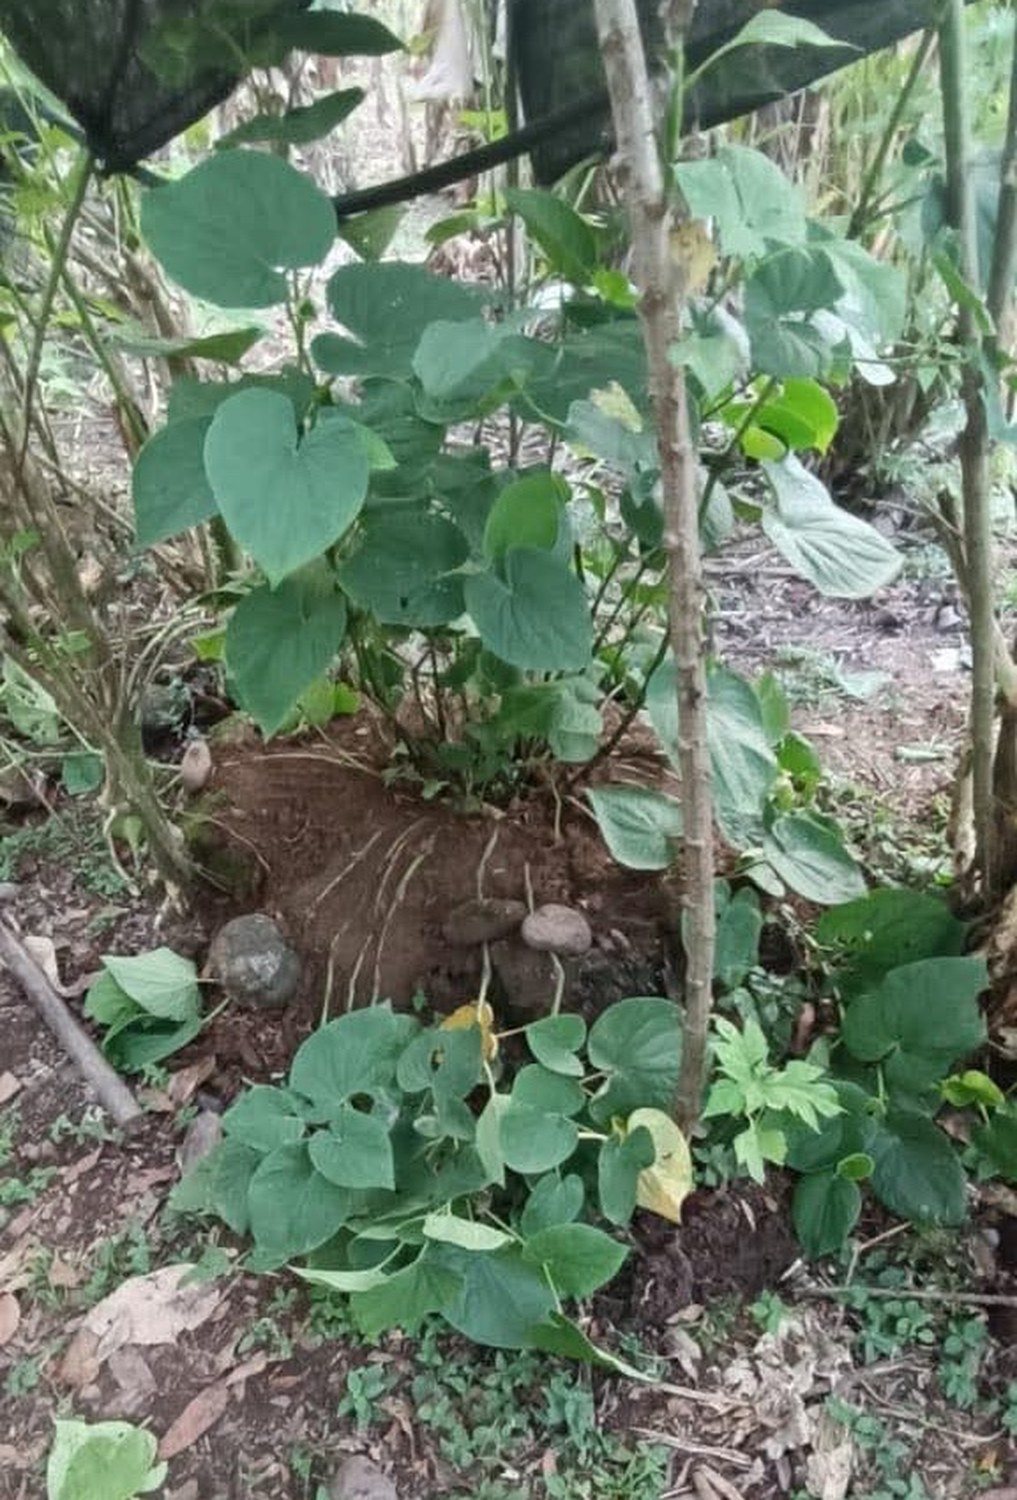
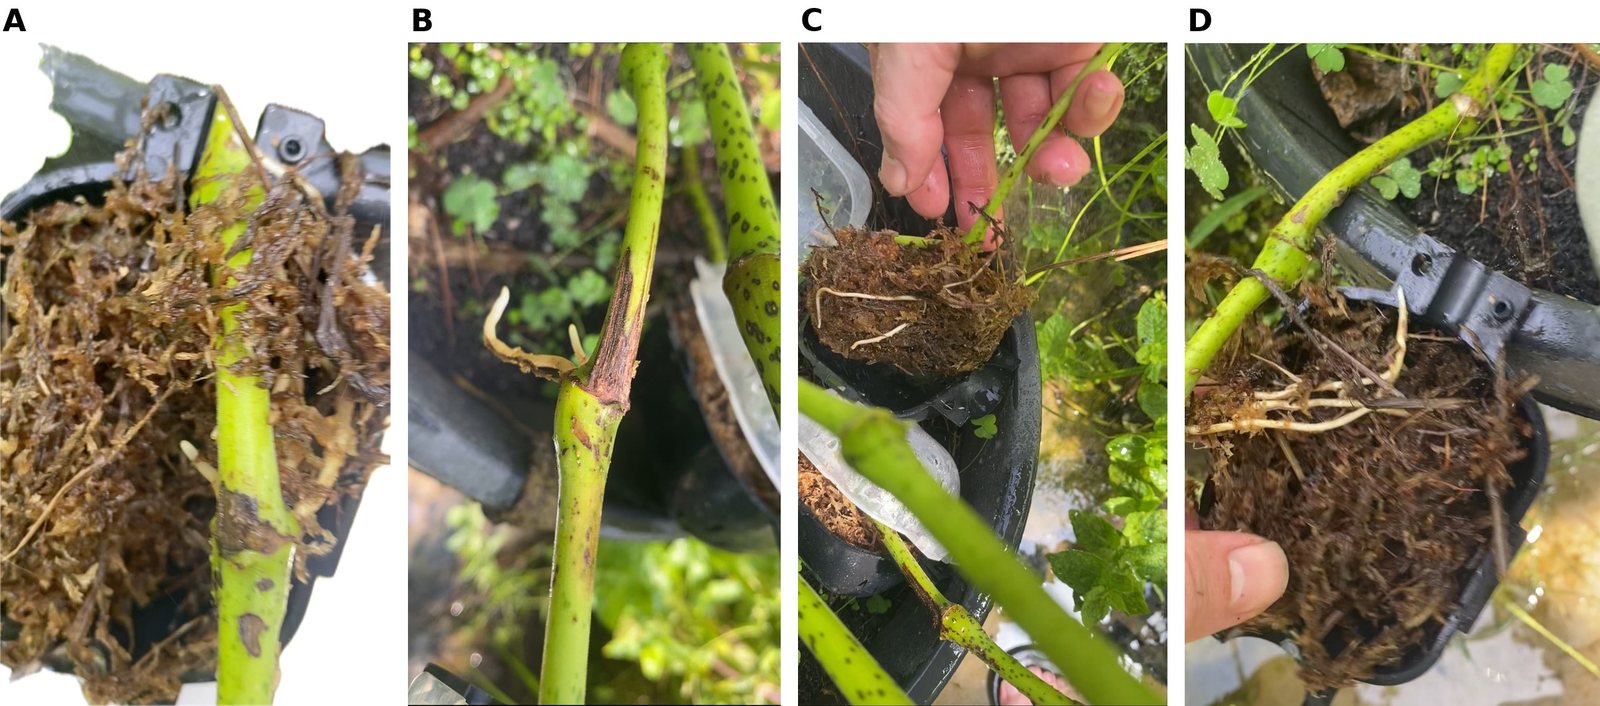
The technique described here draws on two propagation traditions. The first is ground layering, in which lateral stems are bent to contact moistened soil and secured with a stone, inducing adventitious roots at the node–soil interface; in P. nigrum, runners trailed over a raised soil mound root at the nodes and the rooted pieces are then harvested and potted on, giving 90.7% establishment against 62.9% for conventional propagation [6]. Figure 1 shows this practice on a mature kava stool. The second is the Hawaiian practice of propagating kava in moss beds, which the authors have observed in ʻawa cultivation between 2010 and 2025. The present method combines the two: fresh sphagnum moss is inoculated with mycorrhizal and bacterial amendments, packed around hormone-treated nodes, and enclosed in a two-piece pod that creates a stable rooting microenvironment.
This study reports the first systematic, multi-season, outdoor nursery–based assessment of air layering in P. methysticum. Three replicates were conducted over nine months to test whether outcomes were reproducible across contrasting subtropical conditions, using the same four-category rooting scale and 21-day assessment interval applied in the authors' earlier soft-stem work [2] so that results are directly comparable across systems.
2. Related Work
Air layering involves applying exogenous auxin — typically indole-3-butyric acid (IBA) or 1-naphthaleneacetic acid (NAA) — at a node and wrapping the treated zone in a moisture-retentive medium. Outcomes depend on cultivar, stock-plant condition, temperature and moisture during induction, and the physical and biological properties of the rooting medium [7,8]. In guava (Psidium guajava), IBA applied in sphagnum moss and related media produced rooting of up to 85.3% at IBA 6000 ppm, against 52.0% in the untreated control, with sphagnum outperforming cocopeat [9] — although those layers were girdled, unlike the non-wounded nodes used here. In Moringa oleifera, open air layering into seedling plug containers rooted 50% of minimally wounded layers under NAA at 2500 ppm, with all detached layers surviving, while an IBA-based commercial stimulant and a water control did not [10]. No comparable quantitative record exists for kava.
Microbial amendments in propagation substrates have been reported to improve root formation and transplant establishment in a range of tropical crops. Arbuscular mycorrhizal fungi are well documented as contributors to root development and post-transplant vigor [11]. In black pepper — a close relative within the Piperales — soil inoculation with Trichoderma spp., Pseudomonas fluorescens, or arbuscular mycorrhizal fungi significantly increased leaf area, shoot height, root volume, and dry weights of nursery plants relative to an uninoculated control, although combining all three gave no significant additional benefit over the individual inoculants [12]. The inoculated-moss approach used here follows that trajectory. It should be stated plainly that the present study did not include a non-inoculated control and therefore contributes no evidence on whether the microbial component was responsible for any part of the outcome.
Previous kava propagation work under controlled conditions has focused on stem cuttings in soil or aeroponic systems. Blythe et al. [2] reported 47% rooting in peat cubes at 21 days and 51% in aeroponics at 14 days, with the aeroponic approach requiring an indoor, actively managed environment. Broader reviews of clonal propagation of medicinal and aromatic plants reach similar conclusions about the trade-off between infrastructure intensity and throughput [13]. Comparable trade-offs have been quantified in other high-value crops, including Cannabis sativa [14] and in recent aeroponic propagation engineering [15].
Variety selection matters in propagation trials. Kali-ISA and Kali-Hiwa are two commonly grown American kava varieties with observable differences in stem lignification, node spacing, and vigor. Kavalactone concentration varies substantially among kava cultivars grown in a common environment [16], and internode length and stem characteristics differ cultivar by cultivar in the Vanuatu germplasm [5]. These are plausible modifiers of rooting propensity, although the present design cannot attribute any observed difference to a specific trait.
3. Materials and Methods
3.1. Plant Material and Stock Management
Air layers were established on two American kava varieties, "Kali-ISA" and "Kali-Hiwa," obtained from Kali Kava, Sacramento, CA (https://www.KaliKava.com) in October 2024 as tissue-culture-derived nursery stock. Stock plants were propagated under greenhouse conditions at the Kali Kava research nursery in Boca Raton, Florida, then grown on in nursery containers held outdoors on open benches under shade cloth at the same site. All layering reported here was performed on these containerized stock plants under ambient outdoor nursery conditions; the stock plants were not field-planted, and rooted layers were moved to open-field plantings only after detachment, potting, and establishment (Section 4.8). All plants were between 12 and 18 months old at the time of pod installation. Three replicates were conducted in June 2025, October 2025, and February 2026, each using 40 air layers (n = 20 per variety) drawn from the same maintained stock-plant population.
The number of individual stock plants supporting the 120 layers was not recorded, and stock plants were drawn from the same maintained population in all three replicates, so it is likely that some individual plants carried layers in more than one replicate. Neither the number of plants nor the layer-to-plant mapping is available, which constrains the analysis (Section 6). Kali-ISA and Kali-Hiwa are trade designations used in the American kava nursery trade rather than formally registered or morphotype-verified cultivars, and no herbarium vouchers or genetic accessions were deposited. Readers should treat variety identity as provenance-based.
3.2. Air-Layer Preparation
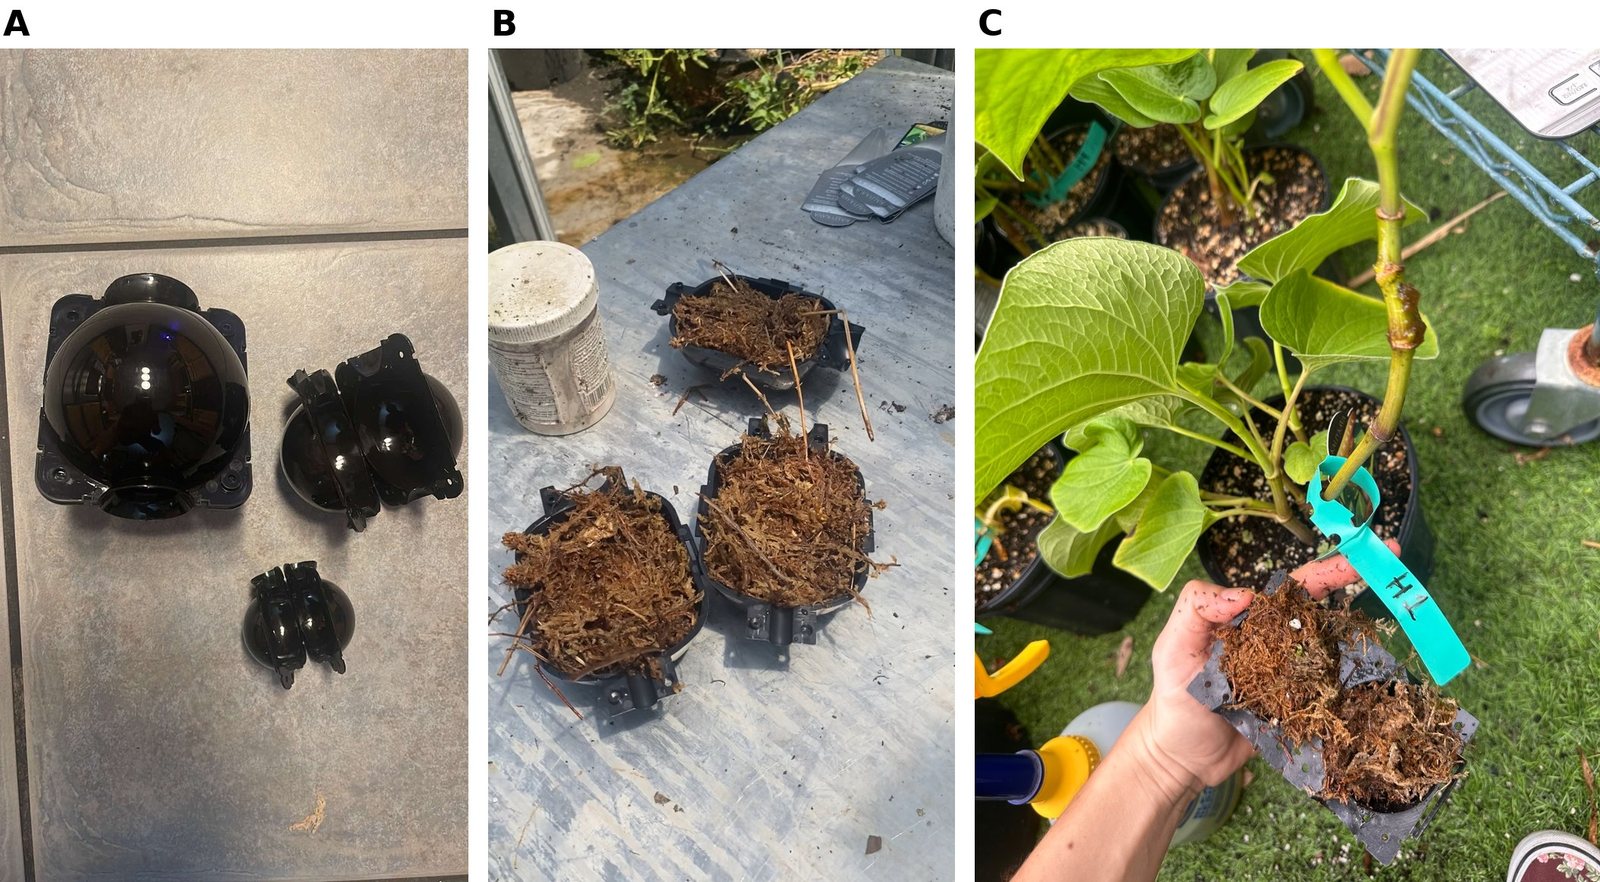
Air layering was performed on intact nodes without wounding or girdling. Stems were selected from the mid-canopy, measuring 0.5–1.0 cm in diameter and corresponding to the first through third node below the apical meristem. Only non-senescing branches with full turgor and uniform dark-green coloration were used. A thin layer of Clonex® Rooting Gel (0.31% w/w indole-3-butyric acid with micronutrients; Growth Technology Ltd, Taunton, UK) was applied directly to the stem surface at the node. Fresh sphagnum moss was pre-hydrated with distilled water and inoculated as described in Section 3.4. Approximately 10–15 g of inoculated moss (fresh weight, saturated but not dripping) was packed around each treated node and enclosed in an opaque black two-piece snap-together polypropylene air-layering pod nominally 4.7 in (approximately 12 cm) in outer diameter, which closed at both ends around the stem.
Layers were installed outdoors on the containerized stock plants under ambient temperature, humidity, and rainfall, with shade cloth and natural canopy shading from adjacent kava foliage reducing desiccation and direct insolation. No greenhouse, propagation chamber, or other controlled-environment enclosure was used at any point during the layering period. Pods were left undisturbed for the full 21-day evaluation period and were not re-watered. Each replicate comprised 40 layers (Kali-ISA n = 20; Kali-Hiwa n = 20). Pods were sanitized between replicates in 10% sodium hypochlorite followed by a clean-water rinse. Layers were not randomized to position, and multiple layers were installed on individual stock plants (see Section 6).
3.3. Propagation Media and Equipment
Live sphagnum moss was obtained from a commercial supplier, Tennessee Wholesale Nursery (tennesseewholesalenursery.com). Air-layer pods were two-piece snap-together polypropylene units of 4.7 in (approximately 12 cm) outer diameter, sourced through a commercial horticultural supplier. No supplemental irrigation, misting, heating, or lighting was applied at any stage of the layering period.
3.4. Rooting Agents and Inoculum Preparation
Rooting gel: Clonex® Rooting Gel, 0.31% w/w indole-3-butyric acid with micronutrients (Growth Technology Ltd, Taunton, UK; distributed in the USA by Hydrodynamics International, Lansing, MI; EPA Reg. No. 79664-1).
Microbial inoculum: a Bacillus root inoculant (Hydroguard®, Botanicare, a brand of The Hawthorne Gardening Company) containing Bacillus amyloliquefaciens at 0.038% w/w, a labeled minimum of 1.0 × 10⁴ CFU mL⁻¹, was applied at 2 mL per gallon (approximately 0.53 mL L⁻¹), together with Plant Success® Great White Premium mycorrhizal inoculant at 3 g per gallon (approximately 0.79 g L⁻¹). The itemized guaranteed analysis for the lot used listed 16 species of mycorrhizal fungi (7 ectomycorrhizal, 9 endomycorrhizal), 12 species of beneficial bacteria plus the yeast Saccharomyces cerevisiae, and 2 Trichoderma species. The manufacturer's marketing copy states 14 bacterial species, which does not reconcile with the itemized list; manufacturer and retailer listings for this product line are not fully consistent, so the composition above should be read as the label statement for the lot used rather than a stable product specification. Both products were combined in 5 gallons (approximately 18.9 L) of distilled water at 25 °C. Sphagnum moss was soaked in this suspension for 4 hours and wrung to a saturated-but-not-dripping moisture level immediately before packing. Inoculum viability was not independently assayed.
3.5. Environmental Conditions
Environmental data were recorded at the Kali Kava Boca Raton nursery throughout each 21-day window using the nursery's existing on-site instrumentation. Values below are reported as observed daily ranges rather than logged means with dispersion statistics; a continuous calibrated data logger was not deployed, and this limits the precision of any climate–outcome inference (Section 6).
Replicate 1 — June 2025 (Summer Wet Season)
Daily highs averaged 33–35 °C (low-to-mid 90s °F) with overnight lows of 24–26 °C (mid-to-upper 70s °F). Relative humidity averaged 80–88%, with frequent afternoon thunderstorms typical of the South Florida wet season. Sustained heat and intermittent heavy rainfall characterized this window.
Replicate 2 — October 2025 (Fall Transitional Season)
Daily highs averaged 27–28 °C (low 80s °F) with overnight lows of 20–23 °C (upper 60s to low 70s °F). Relative humidity averaged 75–80%, with several rain and thunderstorm events in the latter portion of the period. Diurnal humidity swings were modest relative to the summer window.
Replicate 3 — February 2026 (Winter Dry Season)
Daily highs averaged 25–26 °C (upper 70s °F) with overnight lows of 18–19 °C (mid-60s °F). Relative humidity averaged 65–75%, with predominantly dry conditions and intermittent frontal passages. This was the coolest and driest of the three windows.
3.6. Outcome Definitions and Data Collection
At day 21, pods were opened and each layer was assigned to one of four mutually exclusive, exhaustive categories by trained nursery staff working from a common written rubric:
Rotted — complete tissue decay or necrosis at the treated node; no viable tissue.
Alive, no roots — green, turgid stem, with or without new leaf expansion, and no visible root emergence.
Poorly rooted — one or more visible roots, but fewer than three roots reaching 2 cm; this class includes any rooted layer that does not satisfy the well-rooted definition.
Well rooted — three or more roots, each at least 2 cm long, forming a branching root mass.
The "poorly rooted" definition is stated here as a residual class so that the four categories are exhaustive; a layer bearing, for example, two roots of 3 cm is classified as poorly rooted. Layers in the poorly-rooted and well-rooted classes were combined as "total rooted" for success calculations. Root length was measured with a steel rule to the nearest 0.5 cm. Scoring was neither blinded to variety nor independently duplicated, and inter-rater reliability was therefore not established (Section 6).
3.7. Statistical Analysis
Outcomes were recorded as counts and proportions within each category. Binomial proportions are reported with Wilson score 95% confidence intervals. The effect of variety on total rooting success was assessed within each replicate with Fisher's exact test (two-tailed). Pooled across replicates, the variety effect was assessed with a 2 × 2 chi-square test using Yates' continuity correction and, to account for replicate as a stratum, with a Cochran–Mantel–Haenszel test; homogeneity of odds ratios across strata was checked with a test of equal odds. The effect of season was assessed with a 3 × 2 chi-square test on total rooted versus not rooted, pooling varieties. All tests were two-tailed at α = 0.05, and no adjustment for multiplicity was applied. The unit of analysis throughout is the individual air layer, not the stock plant; all reported intervals and p-values assume that layers are independent, which the design does not guarantee (Section 6). Analyses were performed in Python 3 using SciPy 1.18 and statsmodels 0.14.
A post hoc power calculation indicates that, for the observed effect (81.7% versus 70.0%; Cohen's h = 0.274), the achieved power at n = 60 per variety was approximately 0.32, and approximately 209 layers per variety would be required for 80% power at α = 0.05. The study is therefore clearly underpowered for the inter-variety comparison, and the null results below should be read as inconclusive rather than as evidence of equivalence.
Comparisons with previously published propagation outcomes are descriptive. Those studies were not run concurrently, used different plant material and endpoints, and are not controls in any experimental sense. Where a formal test against a fixed reference proportion is given, it is a one-sample binomial test and inherits all of those limitations.
4. Results
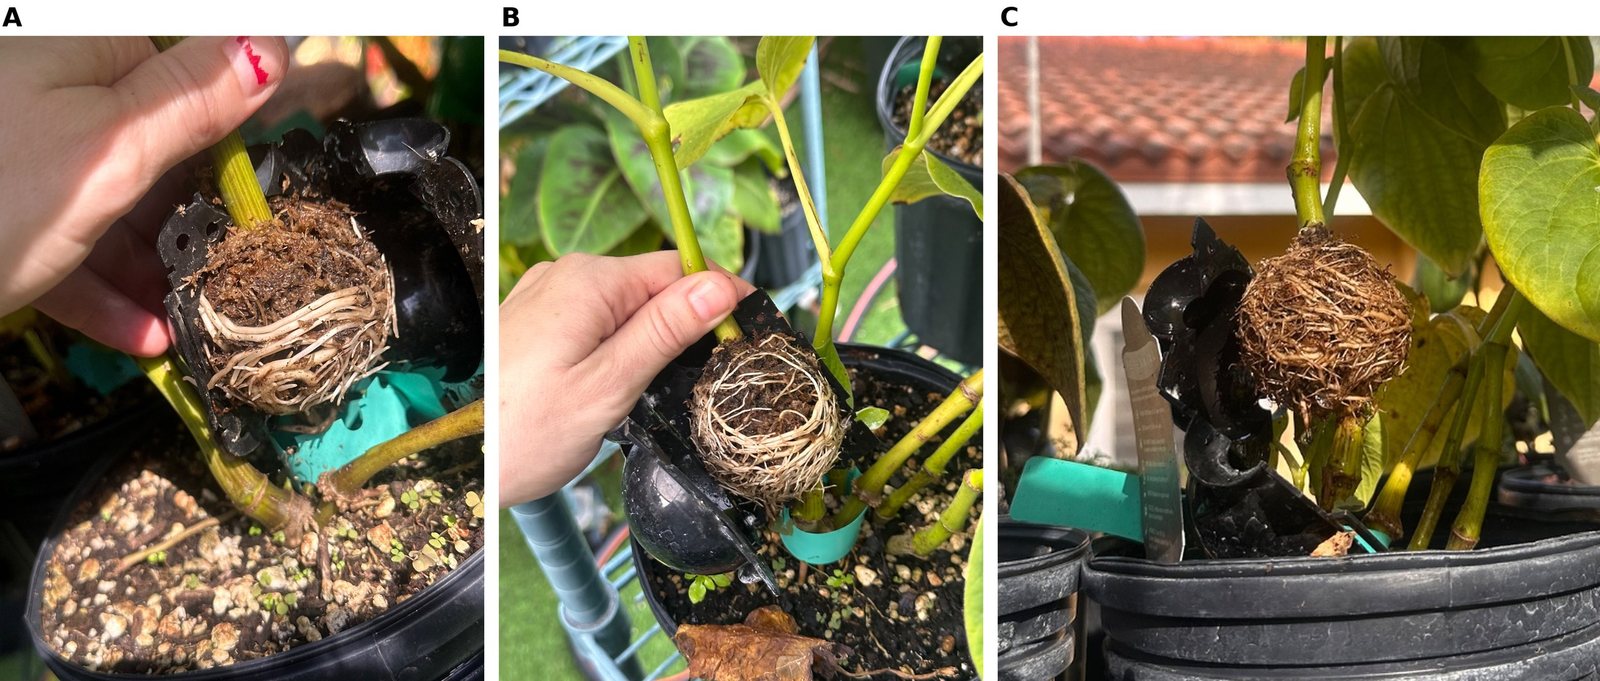
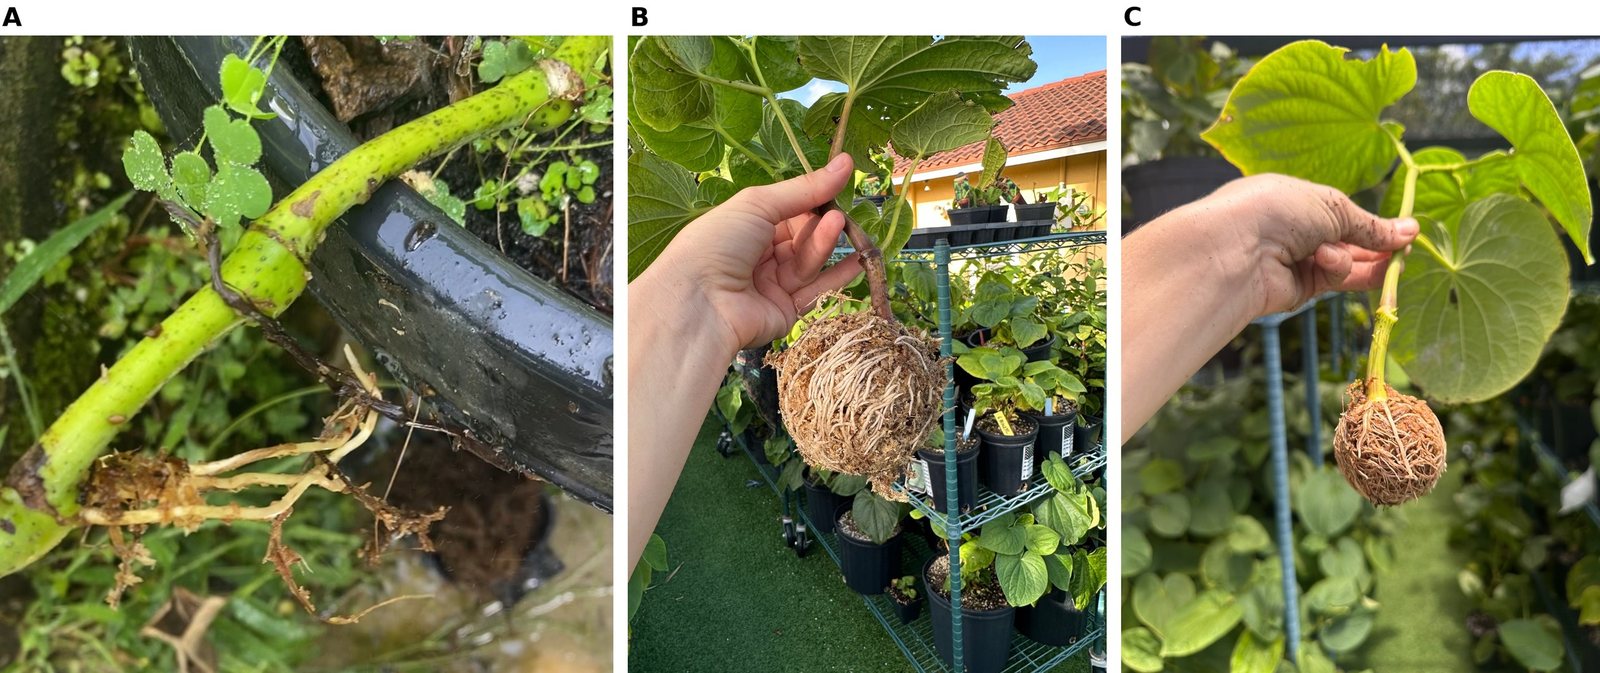
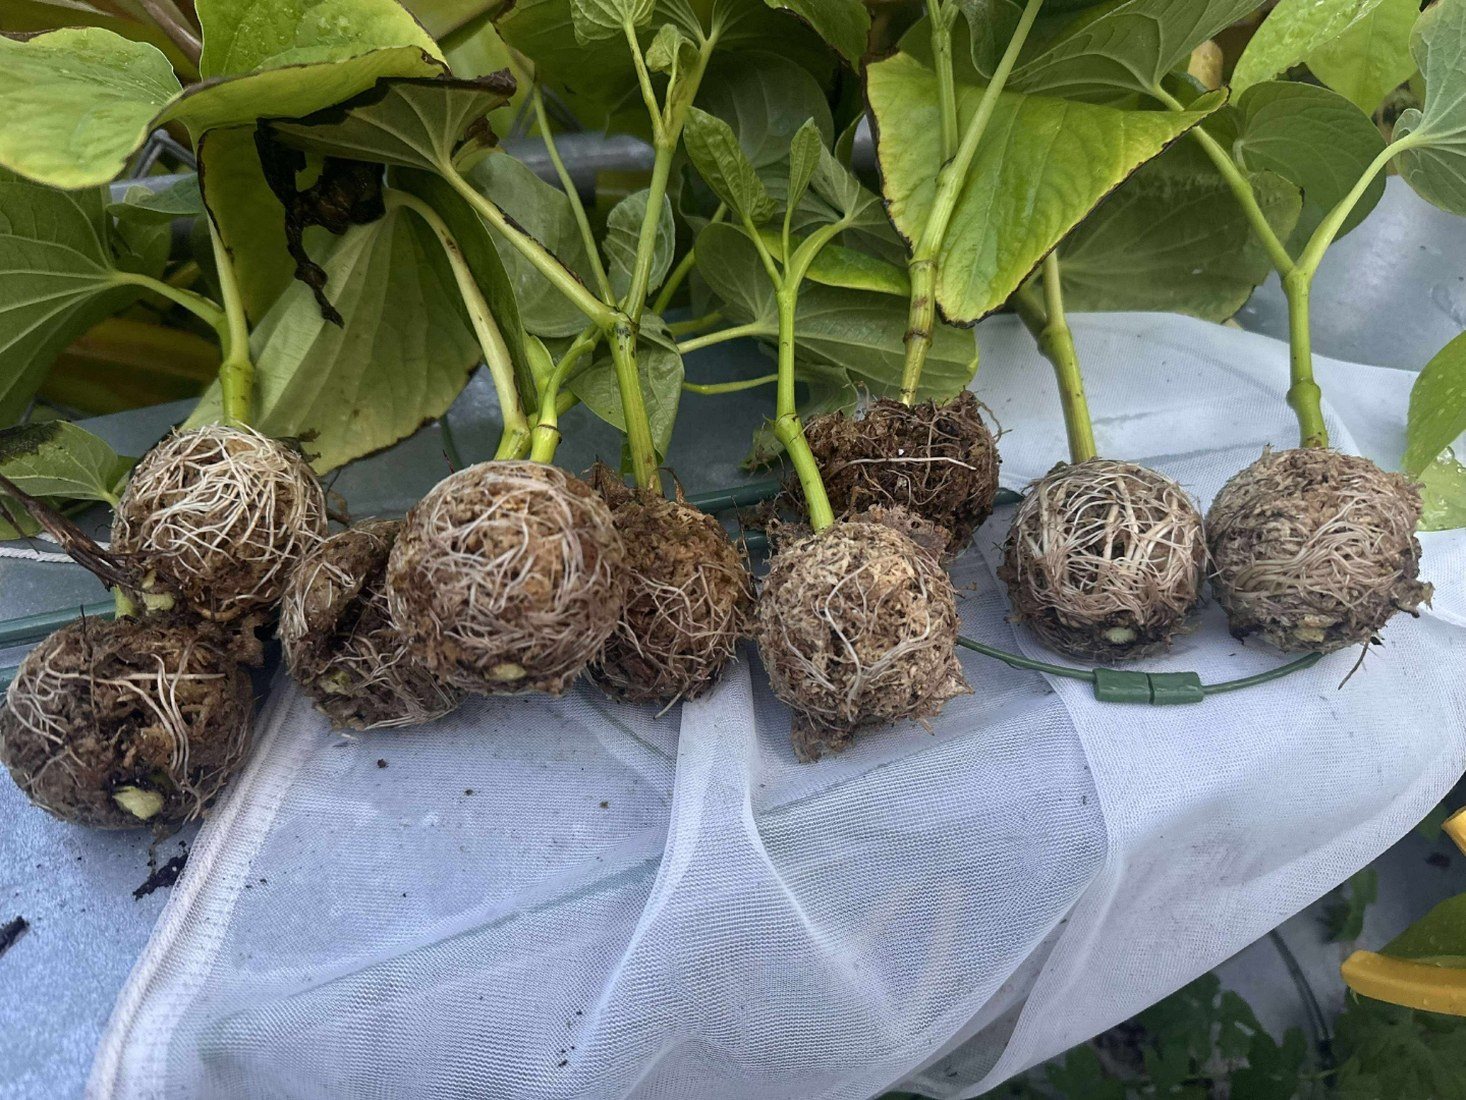
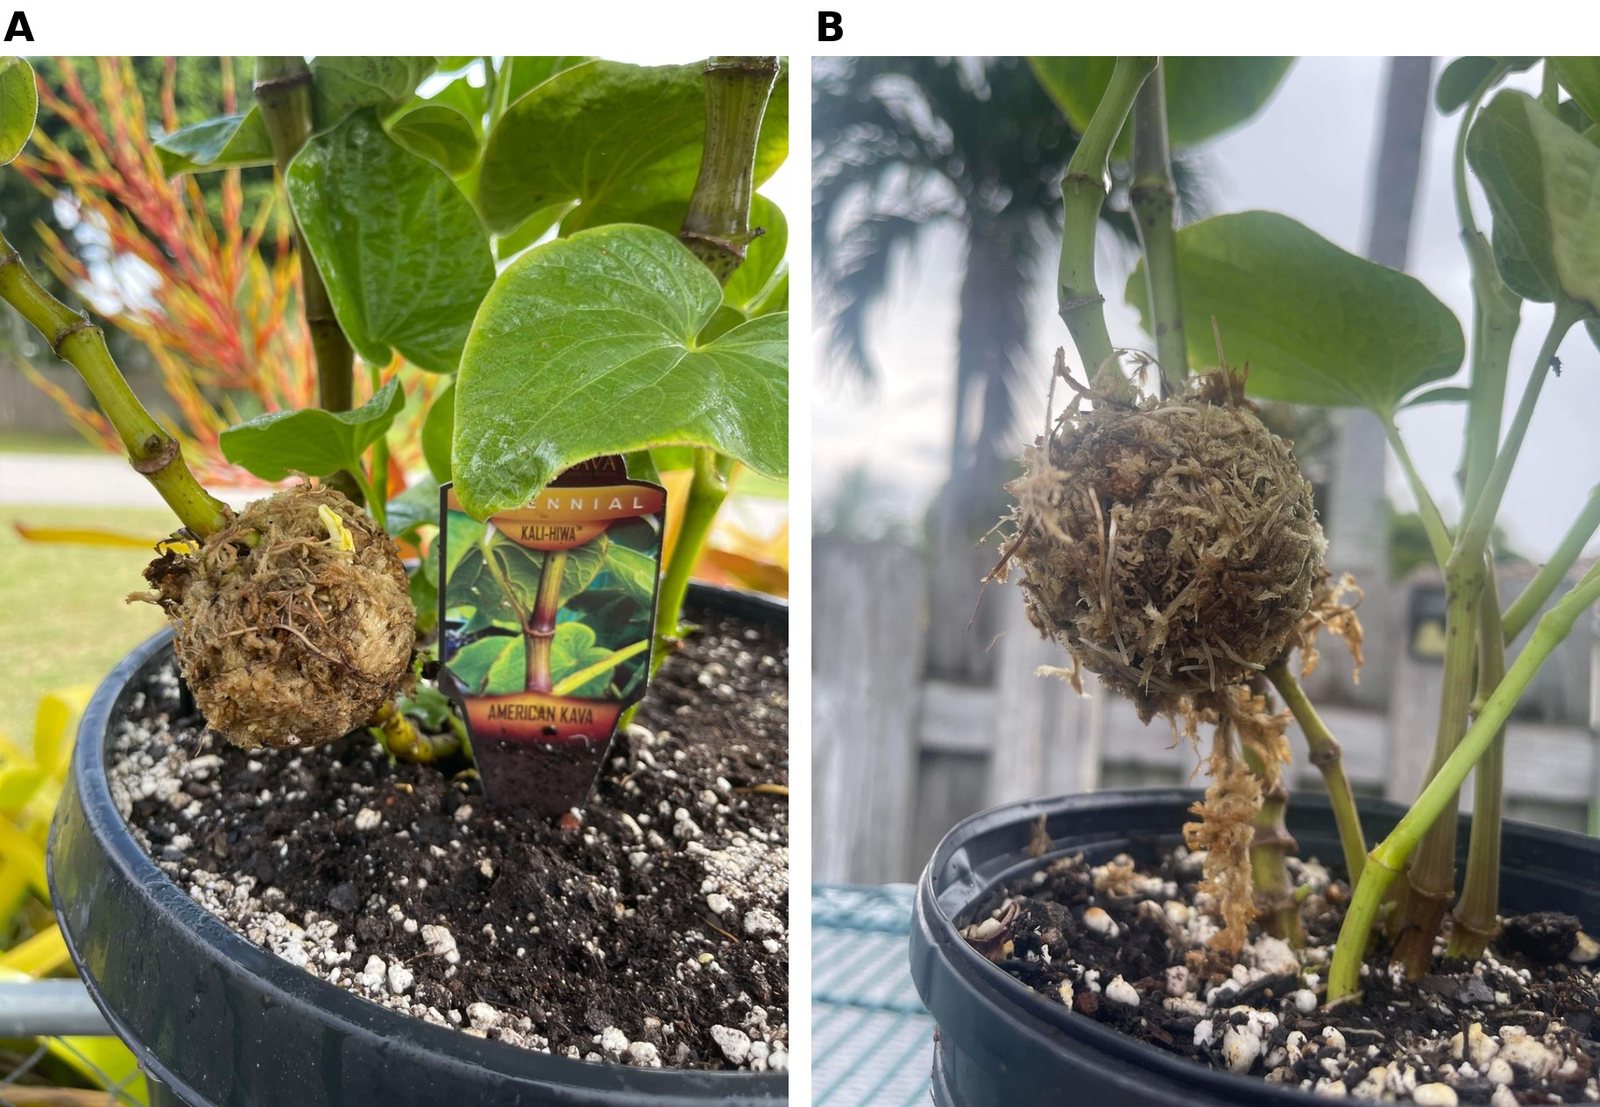
Root formation was observed in both varieties in all three replicates. Results are presented by replicate (Tables 1–3), pooled across replicates (Table 4), and against published benchmarks (Table 5). Figures 4–6 illustrate the rooting classes and the appearance of layers at assessment and detachment; Figures 7 and 8 show the propagules at potting and after transplant.
4.1. Replicate 1 — June 2025
At day 21, 80.0% of Kali-ISA layers (16/20; 95% CI 58.4–91.9) and 70.0% of Kali-Hiwa layers (14/20; 95% CI 48.1–85.5) were rooted, for an aggregate replicate rate of 75.0% (30/40; 95% CI 59.8–85.8). Well-rooted outcomes predominated in Kali-ISA (65.0%), while Kali-Hiwa carried a higher share of poorly rooted layers (20.0%). Rot incidence in this window was 12.5% of layers (5/40), against 7.5% (3/40) in Replicate 2. Fisher's exact test showed no significant variety difference (odds ratio 1.71, p = 0.72).
| Category | Kali-ISA (n = 20) | Kali-Hiwa (n = 20) |
|---|---|---|
| Rotted | 2 (10.0%) | 3 (15.0%) |
| Alive, no roots | 2 (10.0%) | 3 (15.0%) |
| Poorly rooted | 3 (15.0%) | 4 (20.0%) |
| Well rooted | 13 (65.0%) | 10 (50.0%) |
| Total rooted | 16 (80.0%) | 14 (70.0%) |
Fisher's exact test, total rooted vs. not rooted: OR = 1.71, p = 0.72.
4.2. Replicate 2 — October 2025
At day 21, 85.0% of Kali-ISA layers (17/20; 95% CI 64.0–94.8) and 75.0% of Kali-Hiwa layers (15/20; 95% CI 53.1–88.8) were rooted, for an aggregate rate of 80.0% (32/40; 95% CI 65.2–89.5) — the highest absolute value of the three windows. Well-rooted outcomes predominated in both varieties (Kali-ISA 75.0%; Kali-Hiwa 55.0%), and rot incidence was lowest in this replicate (5.0% and 10.0%). Fisher's exact test showed no significant variety difference (odds ratio 1.89, p = 0.69).
| Category | Kali-ISA (n = 20) | Kali-Hiwa (n = 20) |
|---|---|---|
| Rotted | 1 (5.0%) | 2 (10.0%) |
| Alive, no roots | 2 (10.0%) | 3 (15.0%) |
| Poorly rooted | 2 (10.0%) | 4 (20.0%) |
| Well rooted | 15 (75.0%) | 11 (55.0%) |
| Total rooted | 17 (85.0%) | 15 (75.0%) |
Fisher's exact test, total rooted vs. not rooted: OR = 1.89, p = 0.69.
4.3. Replicate 3 — February 2026
At day 21, 80.0% of Kali-ISA layers (16/20; 95% CI 58.4–91.9) and 65.0% of Kali-Hiwa layers (13/20; 95% CI 43.3–81.9) were rooted, for an aggregate rate of 72.5% (29/40; 95% CI 57.2–83.9). Kali-ISA performance was indistinguishable from the summer replicate. Fisher's exact test showed no significant variety difference (odds ratio 2.15, p = 0.48). All three replicate confidence intervals overlap substantially.
| Category | Kali-ISA (n = 20) | Kali-Hiwa (n = 20) |
|---|---|---|
| Rotted | 2 (10.0%) | 3 (15.0%) |
| Alive, no roots | 2 (10.0%) | 4 (20.0%) |
| Poorly rooted | 3 (15.0%) | 3 (15.0%) |
| Well rooted | 13 (65.0%) | 10 (50.0%) |
| Total rooted | 16 (80.0%) | 13 (65.0%) |
Fisher's exact test, total rooted vs. not rooted: OR = 2.15, p = 0.48.
4.4. Rooting Classes at Assessment
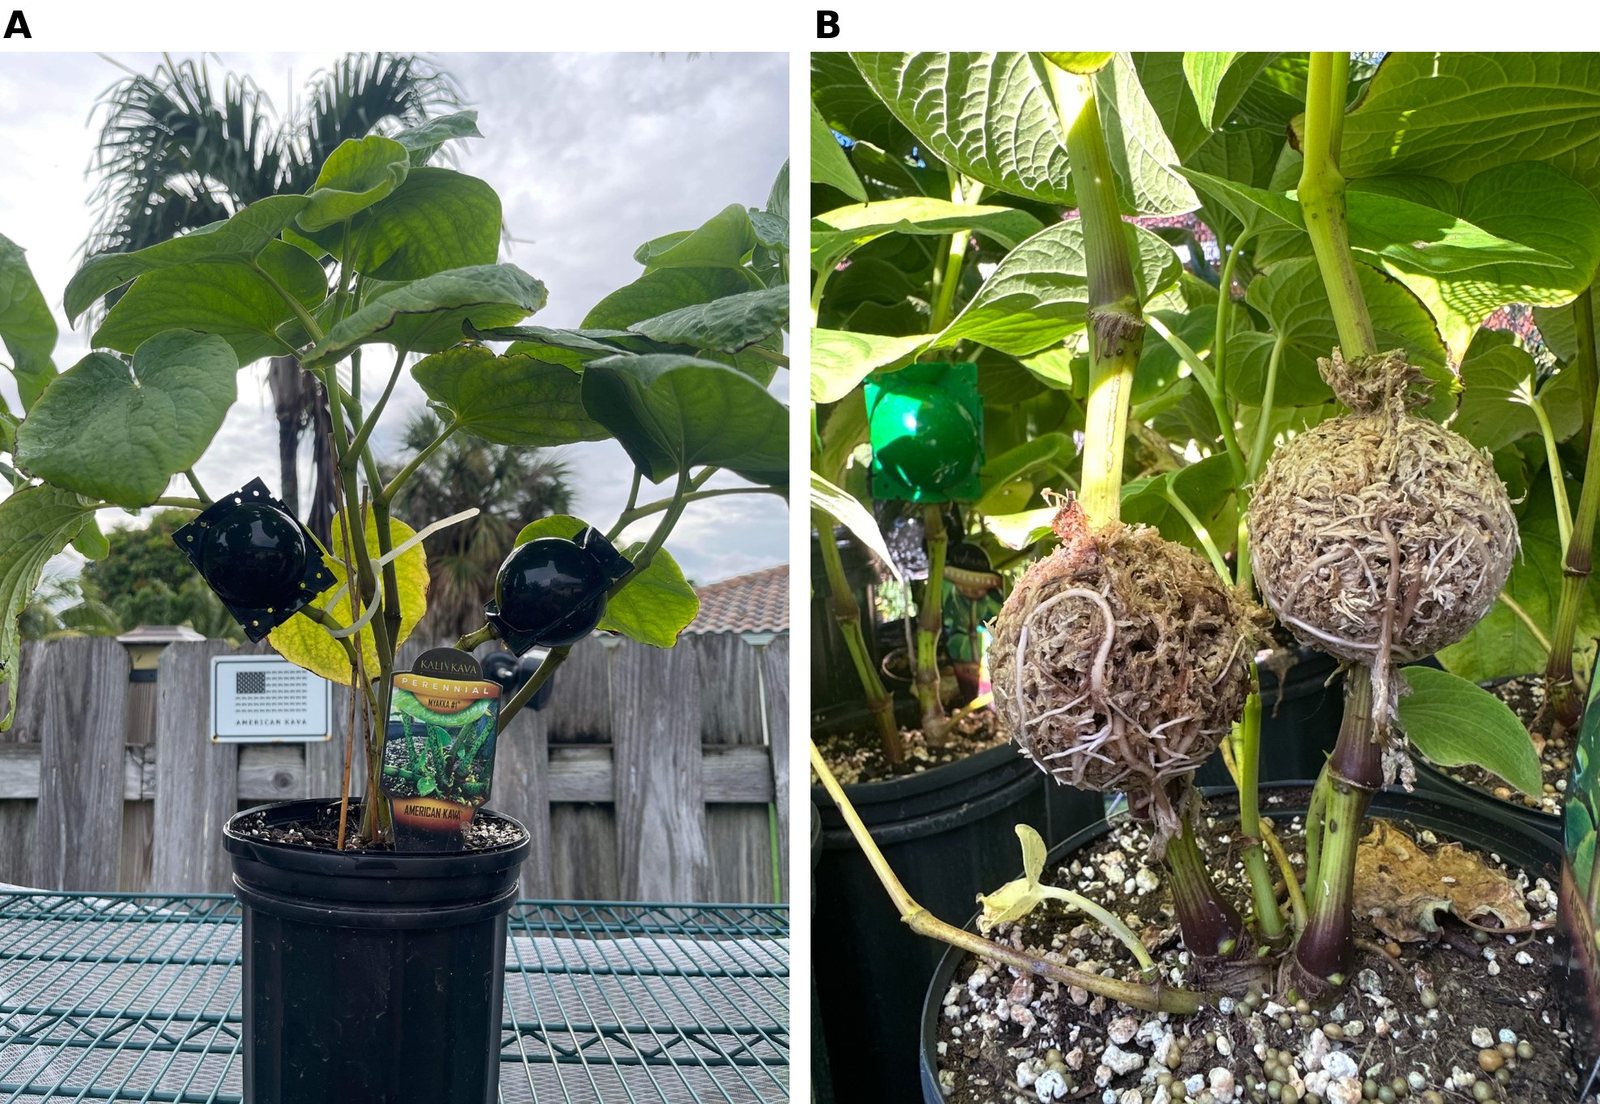
Figure 4 shows representative layers spanning the scoring scale at pod opening, and Figure 5 shows pods opened in situ at day 21 with the stock plant undisturbed. Photographs were selected to illustrate the category definitions and were not drawn by random sampling from the scored units; they are documentary rather than quantitative evidence.
4.5. Pooled Results Across Replicates
Pooled across all three replicates (n = 60 per variety; n = 120 total), Kali-ISA reached 81.7% rooting (49/60; 95% CI 70.1–89.4) and Kali-Hiwa 70.0% (42/60; 95% CI 57.5–80.1), for a combined rate of 75.8% (91/120; 95% CI 67.4–82.6). Well-rooted classifications accounted for 68.3% of Kali-ISA and 51.7% of Kali-Hiwa layers. Rot incidence was low in both varieties (8.3% and 13.3%).
The 11.7 percentage-point pooled difference in favor of Kali-ISA was not statistically significant (Yates-corrected χ² = 1.64, df = 1, p = 0.20; risk difference 11.7 pp, 95% CI −3.5 to +26.8 pp). Stratifying by replicate, the Cochran–Mantel–Haenszel common odds ratio was 1.92 (95% CI 0.81–4.52, p = 0.14), and the test of equal odds across strata was consistent with homogeneity (p = 0.98), indicating that the direction and magnitude of the variety effect were stable across seasons even though the effect itself was not resolvable at this sample size.
| Category | Kali-ISA (n = 60) | Kali-Hiwa (n = 60) | Combined (n = 120) |
|---|---|---|---|
| Rotted | 5 (8.3%) | 8 (13.3%) | 13 (10.8%) |
| Alive, no roots | 6 (10.0%) | 10 (16.7%) | 16 (13.3%) |
| Poorly rooted | 8 (13.3%) | 11 (18.3%) | 19 (15.8%) |
| Well rooted | 41 (68.3%) | 31 (51.7%) | 72 (60.0%) |
| Total rooted | 49 (81.7%) | 42 (70.0%) | 91 (75.8%) |
Total rooted, Kali-ISA vs. Kali-Hiwa: Yates-corrected χ² = 1.64, df = 1, p = 0.20; Mantel–Haenszel common OR = 1.92 (95% CI 0.81–4.52), p = 0.14. Wilson score 95% confidence intervals for total rooted: Kali-ISA 70.1–89.4%; Kali-Hiwa 57.5–80.1%; combined 67.4–82.6%.
4.6. Seasonal Comparison
Aggregate rooting was 75.0% in June 2025, 80.0% in October 2025, and 72.5% in February 2026. A 3 × 2 chi-square test on total rooted versus not rooted, pooling varieties, found no significant difference among the three windows (χ² = 0.64, df = 2, p = 0.73). The confidence intervals for the three replicates overlap almost completely. The correct reading is therefore that the method performed consistently across summer, transitional, and winter conditions — not that October was superior. The ordering of the replicate means is well within sampling variation and is not interpreted further.
4.7. Comparison with Published Benchmarks
Aggregate rooting exceeded the values reported for the alternative systems summarized in Table 5. One-sample binomial tests of the pooled result against each reference proportion return p < 0.001 in every case (91/120 vs. 47%, p = 2 × 10⁻¹⁰; vs. 51%, p = 4 × 10⁻⁸; vs. 60%, p = 4 × 10⁻⁴). These tests treat the published figures as fixed, known constants, which they are not; they are offered only to show that the difference is larger than sampling noise in the present sample, not as evidence of a controlled between-method effect.
Two caveats attach to the nodal-cutting benchmark specifically. First, Davis and Brown [1] report the percentage of cuttings that formed plants — an establishment/emergence endpoint — rather than rooting scored at a fixed interval, so the endpoints are not equivalent. Second, their Table 9 gives 20%, 49%, and 60% for basal, middle, and apical nodes planted in March, and 39%, 60%, and 56% for the same positions planted in August. The full reported range is therefore 20–60%, and citing "49–60%" alone would select the more favorable subset.
| Method / environment | Interval | Scope | Reported outcome | Endpoint and caveats |
|---|---|---|---|---|
| Outdoor container nursery, South Florida — air layering, pooled (present study) | 21 d | 2 American varieties | 75.8% (91/120) 95% CI 67.4–82.6 | Rooting at fixed interval; ambient outdoor nursery; vascular continuity maintained |
| Outdoor container nursery, South Florida — air layering, Oct 2025 (present study) | 21 d | 2 American varieties | 80.0% (32/40) 95% CI 65.2–89.5 | Best single replicate; difference from other replicates not significant (p = 0.73) |
| Greenhouse — soft-stem cuttings in peat cubes [2] | 21 d | 2 American varieties | 47% | Rooting at fixed interval; excised tissue; source internally reviewed, not externally peer reviewed |
| Greenhouse — soft-stem cuttings in aeroponics [2] | 14 d | 2 American varieties | 51% | Shorter interval; high technical and energy input; source internally reviewed, not externally peer reviewed |
| Field, South Pacific — nodal cuttings [1] | To establishment | Multiple Pacific varieties | 20–60% | Cuttings that formed plants, not rooting score; strong node-position and planting-month effects |
4.8. Post-Transplant Establishment
At 21 days, all layers scored as rooted were severed from the mother plants and potted into 1-gallon nursery containers with standard nursery medium (Figure 7), then held under 30% shade cloth at the same site without supplemental humidity control. Across all three replicates and both varieties, 91 of 91 transplanted layers (100%; 95% CI 95.9–100) survived to the 30-day assessment, with no observed transplant shock, wilting, or mortality. Survival was recorded as a binary presence/vigor observation; no growth, biomass, or root-development measurements were taken at that point, and 30 days is too short an interval to speak to establishment in any agronomic sense. Surviving plants were subsequently moved to open-field plantings, but that transfer occurred after the 30-day observation window closed and no field outcomes are reported here.
5. Discussion
Air layering produced consistent rooting in Piper methysticum across three seasonal windows, with an aggregate rate of 75.8% (95% CI 67.4–82.6) at 21 days and replicate rates between 72.5% and 80.0% that were statistically indistinguishable from one another. The technique is well established in other woody and tropical crops, but we found no prior peer-reviewed quantification of it in kava, and the contribution of this work is a standardized measurement under outdoor nursery conditions rather than the invention of a method.
Measured against the available reference points, the outcome is favorable: pooled rooting exceeded the authors' earlier peat-cube (47%) and aeroponic (51%) soft-stem results and the 20–60% establishment range reported for nodal cuttings in the South Pacific. That comparison must be read with care. None of these were concurrent controls; the plant material, climates, endpoints, and assessors differ; the soft-stem figures come from an internally reviewed white paper rather than externally peer-reviewed work; and the nodal-cutting figures measure plant formation rather than rooting. The defensible statement is that air layering performed well in absolute terms under the conditions tested, not that it has been shown to outperform these alternatives in a controlled comparison.
One candidate explanation for the performance observed here is the preservation of vascular continuity with the mother plant, and it is worth being explicit that this runs against the conventional account of adventitious rooting rather than following from it. Auxin is the central regulator of adventitious root formation, acting through auxin canalization to responding target cells and a downstream cascade involving AUX/IAA proteins, TOPLESS, ARFs, and SAUR-like proteins [17,18]. In cuttings, however, the early auxin accumulation that initiates rooting is generally attributed to the interruption of the basipetal auxin drain caused by excision, together with wound signaling [8,18]. On that account an attached layer, which retains its basipetal drain, should have less of an auxin stimulus rather than more, and the applied IBA presumably substitutes for it.
What an attached layer does retain is the resource network that excision removes. Adventitious root formation in cuttings proceeds under isolation from the whole-plant resource and signal network, with wound-induced ethylene and jasmonate signaling, altered auxin conjugation and catabolism, and reduced invertase activity that impairs sink establishment at the rooting zone [18]. A layer continues to receive water and photosynthate from the mother plant throughout induction, which is the more plausible basis for any advantage and is consistent with the fact that no layer required misting or humidity control. The present design tests none of this. No hormone, carbohydrate, or transport measurements were made, and no excised-cutting arm was run in parallel. The account above is a hypothesis for a future factorial experiment, not a finding of this study, and the higher absolute rooting rate reported here is equally consistent with differences in plant material, node selection, substrate, and assessor between this trial and the historical comparators.
Seasonal effects were not detected. October gave the highest point estimate, and June and February the lowest, but the three-way test was clearly null (p = 0.73) and the intervals overlap. Rather than reading a season optimum into the ordering, the useful result is a negative one with practical value: the method did not fail in peak summer heat or in the cool, dry winter window, and rooting stayed above 70% in every replicate. Temperature and moisture during induction are established determinants of adventitious rooting [7], so a season effect may well exist; this study simply lacked the resolution to find one.
Kali-ISA outperformed Kali-Hiwa by 11.7 percentage points in the pooled data, with a consistent direction across all three replicates and a homogeneous stratum-specific odds ratio (common OR 1.92). Neither the pooled chi-square (p = 0.20) nor the stratified test (p = 0.14) nor any within-replicate test reached significance, and the risk-difference interval (−3.5 to +26.8 pp) is compatible with no difference and with a substantial one. With achieved power near 0.32, this is an inconclusive result rather than a negative one. The consistency of direction across all three replicates is suggestive enough to justify a properly powered trial, which would need roughly 209 layers per variety (exact solve 208.6, rounded up).
The auxin gel and microbial inoculum were applied together to every layer. No factorial arms, no auxin-only or inoculum-only treatment, and no untreated control were included. Nothing in these data speaks to the contribution of either input, individually or in combination, and any statement that microbial inoculation improved rooting here would be unsupported. The same applies to the moss substrate and the enclosure: the protocol was evaluated as a package.
From an operational standpoint, air layering shifts investment away from fixed capital and environmental control and toward per-plant labor. At a wage of US$25.00 per hour, installing a layer took approximately 3–10 minutes of hands-on time (US$1.25–4.17), with a further 2–7 minutes to detach and pot a rooted layer (US$0.83–2.92), for 5–17 minutes and US$2.08–7.08 per rooted layer carried through to potting. With pods and moss reconditioned and reused, recurring materials are largely confined to hormone, inoculant, and labeling, at US$0.25–1.10 per layer. Combining the two gives an estimated US$1.50–5.27 per layer installed and US$2.33–8.18 per rooted layer potted (Table 6). These ranges are wide because the site kept two independent time-and-motion records that do not agree: one logged 3–6 minutes per installation and 2–4 minutes per transplant, the other 6–10 and 4–7 minutes. Neither was collected under a stopwatch protocol, so the figures reported here span both records rather than selecting the more favorable one. These are informal observations at research-nursery scale from a single site and crew, not a costed production model; they exclude stock-plant maintenance, overhead, sanitation labor, capital recovery on the pod inventory, and the labor absorbed by layers that fail. They should not be used for commercial planning without validation at production scale.
| Category | Component | Time low (min) | Time high (min) | Cost low | Cost high | Notes |
|---|---|---|---|---|---|---|
| LABOR — costed at US$25.00/hr | ||||||
| Labor | Air-layer installation | 3 | 10 | US$1.25 | US$4.17 | Node selection, hormone application, moss packing, pod closure |
| Labor | Detachment and transplant | 2 | 7 | US$0.83 | US$2.92 | Potting and watering-in; applies to rooted layers only |
| Labor | Total labor per rooted layer potted | 5 | 17 | US$2.08 | US$7.08 | Installation plus detachment |
| MATERIALS — per air layer installed | ||||||
| Consumables | Rooting hormone (IBA gel, ~0.1 mL) | — | — | US$0.03 | US$0.10 | Per-node application |
| Consumables | Microbial inoculants (AMF + bacteria) | — | — | US$0.10 | US$0.50 | Prorated dose from bulk suspension |
| Consumables | Fasteners, labels, sanitation | — | — | US$0.05 | US$0.30 | Hypochlorite, ties, tags |
| Consumables | Subtotal — consumables | — | — | US$0.18 | US$0.90 | Excludes reusable components |
| Reusables (amortized) | Air-layer pod | — | — | US$0.05 | US$0.15 | Assumes 10–20 reuse cycles; sanitized between replicates |
| Reusables (amortized) | Sphagnum moss charge (10‑15 g) | — | — | US$0.03 | US$0.10 | Reconditioned and reused |
| Reusables (amortized) | Subtotal — reusables | — | — | US$0.08 | US$0.25 | Sanitization labor not monetized |
| Materials | Total material cost | — | — | US$0.25 | US$1.10 | Per air layer installed |
| TOTALS | ||||||
| Total per air layer installed | Installation labor + all materials | 3 | 10 | US$1.50 | US$5.27 | Low = low labor + low materials; high = high + high |
| Total per rooted layer potted | Total labor + all materials | 5 | 17 | US$2.33 | US$8.18 | Cost of one layer only; excludes inputs absorbed by failed layers |
Excluded from all figures: stock-plant maintenance, facility overhead, capital recovery on pod inventory, sanitation labor, and the inputs absorbed by the approximately 24% of layers that did not root. The final row therefore costs one layer through to potting rather than the full production cost of obtaining one rooted plant. Success-adjusting the installed cost — dividing by the 75.8% pooled rooting rate — gives approximately US$1.98–6.95 per rooted layer before detachment labor, and adding detachment labor gives approximately US$2.81–9.87 per rooted plant potted.
Rooted propagules were straightforward to detach and pot, and all survived to 30 days. That is a useful signal of handling robustness, but 30-day survival under shade cloth is a weak proxy for agronomic performance. Whether early rooting vigor translates into comparable growth rate, root-mass development, kavalactone accumulation, or harvestable yield relative to plants raised from cuttings or tissue culture is untested here and is the single most consequential open question for anyone considering the method commercially.
6. Limitations
This is a multi-season proof of concept, and its design constrains what may be concluded from it.
Single site. All three replicates were run at one nursery, the Kali Kava facility in Boca Raton, Florida. Site, soil, canopy, crew, and stock-plant genetics are fully confounded with the reported outcome. Nothing here establishes performance at any other location.
No concurrent control or comparator arm. The study includes no untreated node, no auxin-only or inoculum-only arm, and no parallel cutting-propagation arm. Every comparison to another method is against historical published figures with different endpoints, materials, and assessors. The protocol was tested as an undifferentiated package.
Pseudoreplication. Multiple layers were installed on individual stock plants (Figure 3), so layers are not fully independent observations. Neither the number of stock plants used nor the layer-to-plant mapping was recorded, so within-plant clustering cannot be modeled retrospectively. Because the same stock-plant population served all three replicates, individual plants may also have carried layers in more than one window, so the replicates are not fully independent of one another either. Confidence intervals and p-values reported here assume independence and are therefore likely anti-conservative; the true intervals are wider than stated, and the effective sample size is smaller than n = 120.
Underpowered for the variety comparison. At n = 20 per variety per replicate and n = 60 pooled, achieved power for the observed effect was approximately 0.32. The non-significant variety results are inconclusive, not evidence of equivalence. Approximately 209 layers per variety would be needed for 80% power.
No randomization and no blinding. Layers were not randomized to canopy position or plant, and scoring was performed by nursery staff who were aware of variety identity and who had also installed the layers. Categories 3 and 4 involve judgment at the margin. No layer was scored independently by a second assessor, so inter-rater reliability was not established and observer bias cannot be excluded.
Limited germplasm. Only two varieties were tested, both trade designations from a single supplier, without voucher specimens or genetic verification. Results should not be generalized to P. methysticum broadly or to Pacific germplasm.
Environmental data are descriptive. Conditions were recorded as observed daily ranges from existing nursery instrumentation, not as continuously logged, calibrated series with dispersion statistics. Any climate–outcome inference is correspondingly weak, and the null seasonal result should not be over-read either.
Short follow-up. Post-transplant assessment extended to 30 days and recorded survival only. No growth, biomass, root architecture, or phytochemical measurements were taken, and no long-term field performance data exist for these propagules.
Cost figures are indicative. Labor times are informal observations from one crew at research scale. Material costs assume 10–20 pod reuse cycles that were not verified over a full service life. Overheads and failure costs are excluded.
Self-referential benchmark. The peat-cube and aeroponic comparison figures come from the authors' own manuscript, which remains in review. Until it is published and independently assessable, those comparisons should carry reduced weight.
7. Future Work
The most valuable next experiment is a properly powered factorial trial. At approximately 209 layers per variety, crossed arms of auxin (present/absent) and microbial inoculum (present/absent) would resolve both the variety question and the contribution of each input, which the present design cannot address. Adding a concurrent nodal-cutting arm scored on the same scale by the same blinded assessors would convert the benchmark comparison from historical to controlled.
Multi-site replication across subtropical and tropical environments — including Pacific Island and continental American growing regions — is needed before the method can be described as generally applicable. Trials should record layer position on the stock plant so that within-plant clustering can be modeled with mixed-effects or GEE methods rather than assumed away, and should deploy calibrated continuous environmental logging so that any season or microclimate effect can actually be estimated.
Germplasm breadth should be expanded beyond two trade varieties, with vouchered accessions and recorded morphological covariates — stem diameter, internode length, node position, tissue maturity — so that variety-specific recommendations can be grounded in traits rather than names. Physical and biological parameters of the system (hormone concentration, inoculant composition, moss type and volume, pod size and opacity) merit systematic optimization.
Finally, long-term follow-up is needed. Cohorts should be tracked from transplant through to harvest and assayed for root biomass and kavalactone content alongside plants raised from cuttings and tissue culture, and the economic model should be rebuilt from audited production-scale data rather than research-nursery observation.
8. Conclusion
Across three seasonal replicates in June 2025, October 2025, and February 2026, air layering rooted 75.8% of kava layers (91/120; 95% CI 67.4–82.6) at 21 days, with replicate rates of 72.5–80.0% that did not differ significantly from one another. Kali-ISA rooted at a higher rate than Kali-Hiwa in every replicate, but the pooled 11.7-point difference was not statistically significant and the study was underpowered to resolve it. All 91 rooted layers survived to 30 days after transplant.
These results indicate that air layering can be carried out on containerized stock plants under ambient outdoor nursery conditions in a subtropical climate — without greenhouse, misting, or other controlled-environment infrastructure, without destroying mother-plant biomass, and with predictable per-plant labor — and that rooted layers can subsequently be potted on and moved to open-field plantings. They do not, on this design, establish that air layering is superior to cuttings or aeroponics, that the microbial inoculant contributed to the outcome, that any season is preferable, or that the varieties differ. Each of those questions requires a controlled, adequately powered, multi-site trial. What this study supports is a narrower and still useful claim: under the conditions tested, the method worked reliably enough to justify that larger investigation.
Author Contributions
T.B. conceived the study, designed the protocol, performed the statistical analysis, and drafted the paper. B.M. performed the majority of the air-layer installations and contributed to layer scoring and transplant handling. J.B. maintained the stock-plant population, installed and scored air layers, recorded environmental data at the Kali Kava Boca Raton nursery, and contributed to transplant assessment. All authors reviewed and approved the final paper.
Data Availability
The complete unit-level scoring records for all 120 air layers, the environmental observation logs for the three replicate windows, and the analysis scripts used to generate every statistic reported here are available from the corresponding author on reasonable request. Summary tables are reproduced in full in Tables 1–6.
Use of Generative Artificial Intelligence
Generative artificial intelligence was used in the preparation of this manuscript. Claude Opus 4.6 (Anthropic) was used to compile study data into tabular form, to construct the manuscript tables, and to perform arithmetic checks of the reported calculations. All compiled values and derived calculations were independently verified by the authors against the source records. ChatGPT 5.2 (OpenAI) was used for grammar and language editing only. No data were generated, imputed, or interpreted by generative artificial intelligence.
Funding and Conflicts of Interest
No external funding was received for this research. This paper is published by the American Kava Association. The corresponding author is affiliated with Root of Happiness, Las Vegas, NV, a commercial kava retailer, and holds an interest in Kali Kava, a commercial kava nursery; the remaining authors are affiliated with Nakamal at Home, Boca Raton, FL, also a commercial kava retailer. The Kali-ISA and Kali-Hiwa plant material was supplied by Kali Kava, Sacramento, CA, and all three replicates were conducted at the Kali Kava research nursery in Boca Raton, FL. The authors' employing organizations are therefore distinct from the facility at which the work was carried out, and the trial site is a facility in which the corresponding author holds a commercial interest. These relationships are disclosed as potential conflicts of interest. No manufacturer of any product named in this paper provided funding, materials, or input into the design, conduct, analysis, or reporting of the study.
Supplementary Materials
Supplementary files are available from the corresponding author on reasonable request.
Institutional Review Board Statement
Not applicable. This study did not involve humans or animals.
Informed Consent Statement
Not applicable.
Acknowledgments
The authors thank the Kali Kava nursery staff in Boca Raton who assisted with plant maintenance across the three replicate windows, and acknowledge the Hawaiian ʻawa cultivators whose moss-bed propagation practice informed the design of this method.
Editorial process
Tyler Blythe is the founder of the American Kava Association, which publishes this journal, and is the journal's Editor-in-Chief; he handled this manuscript. Before acceptance the manuscript underwent Computational Manuscript Review (CMR; see editorial policies) and was then accepted on the editor's decision. No editorial review independent of the authors took place. Corrections, if any, are issued as dated notices linked from this page; the version of record is not amended silently.
References
Reference [2] is an American Kava Association technical white paper. It was internally reviewed and audited by the authors but has not been externally peer reviewed, and findings attributed to it should be read on that basis.
- Davis, R.I.; Brown, J.F. Kava (Piper methysticum) in the South Pacific: Its Importance, Methods of Cultivation, Cultivars, Diseases and Pests; ACIAR Technical Reports Series No. 46; Australian Centre for International Agricultural Research: Canberra, Australia, 1999. https://www.aciar.gov.au/publication/technical-publications/kava-piper-methysticum-south-pacific
- Blythe, T.; Bowman, J.; Masifilo, M. Soft-Stem Propagation of Piper methysticum Using Peat-Based Media and Aeroponic Cloning Systems; American Kava Association Technical White Paper No. 1, Version 1.0; American Kava Association: Las Vegas, NV, USA, 2026. https://www.americankavaassociation.org/study/aeroponic-cloning-peat
- Zhang, Z.; Zhao, L.; Chen, X.; Zheng, X. Successful micropropagation protocol of Piper methysticum. Biol. Plant. 2008, 52, 110–112. https://doi.org/10.1007/s10535-008-0020-9
- Prasad, R.; Tyagi, A.P.; Taylor, M. Regeneration and establishment of whole plants from kava (Piper methysticum Forster) meristems in tissue culture. S. Pac. J. Nat. Sci. 2008, 26, 39–44. https://repository.usp.ac.fj/id/eprint/1490/
- Lebot, V.; Cabalion, P. Kavas of Vanuatu: Cultivars of Piper methysticum Forst.; Technical Paper No. 195; South Pacific Commission: Nouméa, New Caledonia, 1988. https://horizon.documentation.ird.fr/exl-doc/pleins_textes/divers14-07/26842.pdf
- Khandekar, R.G.; Haldankar, P.M.; Pande, V.S.; Joshi, G.D.; Bagade, D.S.; Malve, D.B.; Bhagwat, N.R.; Rangwala, A.D.; Jambhale, N.D.; Ramana, K.V. Studies on rapid multiplication of black pepper (Piper nigrum L.) on soil mound. J. Spices Aromat. Crops 2004, 13, 34–36.
- Hartmann, H.T.; Kester, D.E.; Davies, F.T.; Geneve, R.L.; Wilson, S.B. Hartmann & Kester’s Plant Propagation: Principles and Practices, 9th ed.; Pearson: New York, NY, USA, 2018.
- de Klerk, G.-J.; van der Krieken, W.; de Jong, J.C. The formation of adventitious roots: New concepts, new possibilities. In Vitro Cell. Dev. Biol. Plant 1999, 35, 189–199. https://doi.org/10.1007/s11627-999-0076-z
- Punasya, A.; Kanwar, J.; Dubey, R. IBA and rooting media influenced survival, rooting and vegetative growth in air layering of guava (Psidium guajava L.) cv. L-49. Int. J. Curr. Microbiol. Appl. Sci. 2018, 7, 1505–1510. https://doi.org/10.20546/ijcmas.2018.708.171
- Coles, Z.S.; du Toit, E.S. Open air-layering of Moringa oleifera utilizing seedling plug containers. S. Afr. J. Bot. 2020, 129, 225–228. https://doi.org/10.1016/j.sajb.2019.07.016
- Smith, S.E.; Read, D.J. Mycorrhizal Symbiosis, 3rd ed.; Academic Press: London, UK, 2008.
- Kodithuwakku, R.D.; Wijekoon, W.M.R.W.B.; Kumari, I.S.; De Silva, D.P.P. Efficacy of single and combined application of Trichoderma spp. and Pseudomonas fluorescens along with bio-fertilizer (arbuscular mycorrhizae) on growth of nursery plants of black pepper (Piper nigrum L.). Sri Lanka J. Food Agric. 2016, 2, 69–72. https://doi.org/10.4038/sljfa.v2i1.26
- Waman, A.A.; Smitha, G.R.; Bohra, P. A review on clonal propagation of medicinal and aromatic plants through stem cuttings for promoting their cultivation and conservation. Curr. Agric. Res. J. 2019, 7, 122–138. https://doi.org/10.12944/CARJ.7.2.01
- Weingarten, M.; Mattson, N.; Grab, H. Evaluating propagation techniques for Cannabis sativa L. cultivation: A comparative analysis of soilless methods and aeroponic parameters. Plants 2024, 13, 1256. https://doi.org/10.3390/plants13091256
- Tang, L.; Syed, A.-u.-A.; Otho, A.R.; Junejo, A.R.; Tunio, M.H.; Hao, L.; Asghar Ali, M.N.H.; Brohi, S.A.; Otho, S.A.; Channa, J.A. Intelligent rapid asexual propagation technology — A novel aeroponics propagation approach. Agronomy 2024, 14, 2289. https://doi.org/10.3390/agronomy14102289
- Lebot, V.; McKenna, D.J.; Johnston, E.; Zheng, Q.Y.; McKern, D. Morphological, phytochemical, and genetic variation in Hawaiian cultivars of ʻawa (kava, Piper methysticum, Piperaceae). Econ. Bot. 1999, 53, 407–418. https://doi.org/10.1007/BF02866720
- Pacurar, D.I.; Perrone, I.; Bellini, C. Auxin is a central player in the hormone cross-talks that control adventitious rooting. Physiol. Plant. 2014, 151, 83–96. https://doi.org/10.1111/ppl.12171
- Druege, U.; Franken, P.; Hajirezaei, M.R. Plant hormone homeostasis, signaling, and function during adventitious root formation in cuttings. Front. Plant Sci. 2016, 7, 381. https://doi.org/10.3389/fpls.2016.00381
How to cite
Blythe, T.; Bowman, J.; McDonnell, B. Outdoor Nursery Propagation of Kava (Piper methysticum) by Air Layering. J. Am. Kava 2026, 1, 004. https://journalofamericankava.org/articles/air-layering-florida
Please cite this version of record. The earlier preprint (10.5281/zenodo.22838843) is superseded by it.